
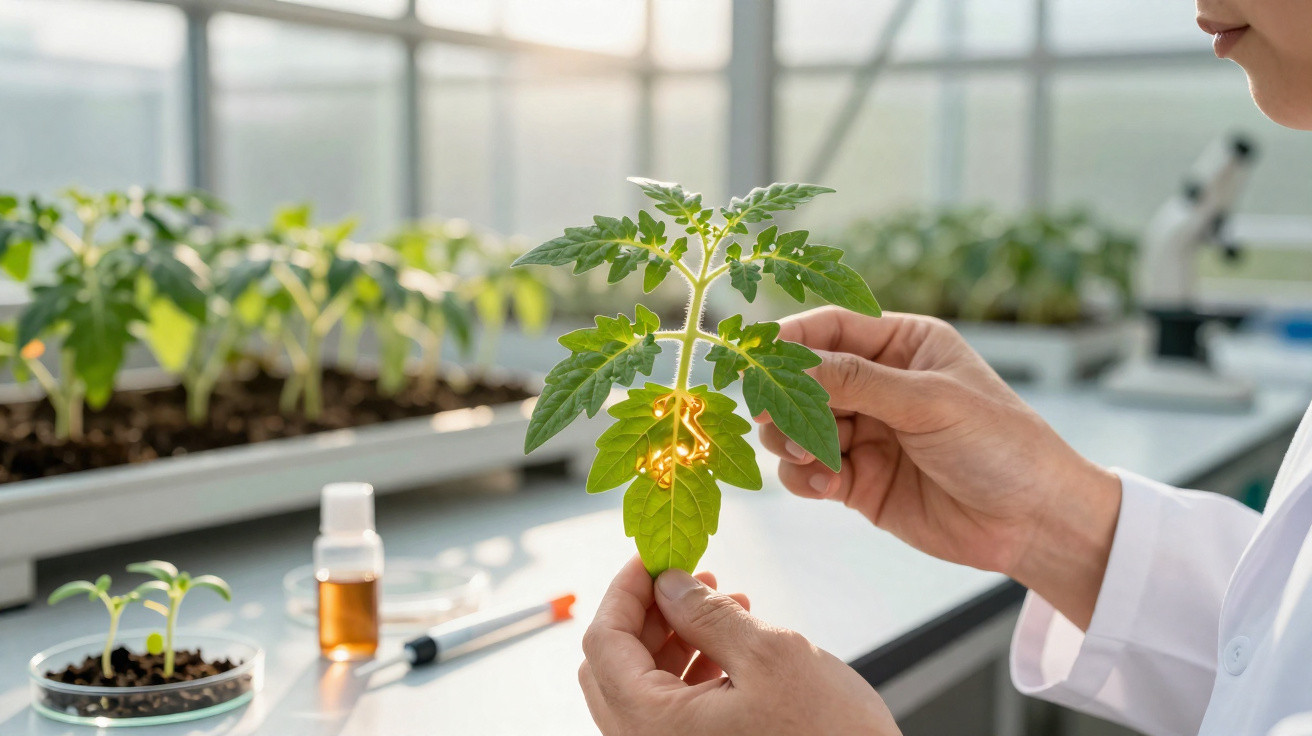
A tomato plant produces every leaf through a defined sequence. First, it identifies the position for a new leaflet, before allowing that location to develop into a complete blade.
A single hormone, auxin, governs both stages. Yet it had remained unclear how one signal could both initiate a leaflet and subsequently cause it to enlarge.
The auxin and gibberellin hormone puzzle
Within plants, auxin seldom works by itself. Under most circumstances, it increases levels of the second growth hormone, gibberellin, meaning that both hormones generally encourage growth together.
That established relationship made tomato leaves particularly puzzling. If auxin always boosted gibberellin, it seemed unable to perform the opposing jobs of starting a leaflet and then promoting its later growth.
Researchers led by Dr Alon Israeli therefore examined the two hormones as leaves formed. The study was carried out in Professor Naomi Ori’s laboratory at the Hebrew University of Jerusalem.
“The same hormone has to accomplish two very different tasks during organ formation,” said Ori.
Following hormones during leaf development
Tomato provided a useful system for the investigation. Its leaves are divided into numerous small leaflets, with every new leaflet identifying a site at which part of the leaf begins to develop.
The researchers treated young leaves with picloram, a synthetic auxin. They then examined which genes were activated and which were switched off.
They also studied mutant plants. In one mutant, the auxin signal is weakened and leaves show little response; in another, the signal continues for much longer than usual.
The prolonged-signal mutant was especially important. Because its leaves behave as though auxin is constantly present, it allowed the team to observe the effects of a sustained signal.
Gibberellin drops before rising again
A brief auxin pulse produced an unexpected effect. In just 10 minutes, it activated genes that break down gibberellin while reducing the activity of genes responsible for producing it.
Gibberellin fell right where a new leaflet was about to form. That local drop, not a rise, is what allowed the leaflet to begin.
Then the whole pattern reversed. In plants with a long-running auxin signal, gibberellin-making genes switched on instead, and levels rose again while the blade expanded outward.
The key, then, was timing. A short-lived signal reduced gibberellin to initiate a leaflet, whereas a prolonged signal increased it to support growth.
Genes activated at the earliest stage
The genes that break down gibberellin were not activated across the entire leaf. Instead, they became active precisely at the sites where new leaflets were beginning to emerge.
A separate gibberellin-making gene behaved the opposite way. It stayed active in the broad, growing regions of the leaf, where blades widened.
The two groups of genes therefore divided the work within the leaf. One reduced gibberellin at the small initiation sites, while the other maintained high levels in tissue that needed to expand.
Mutant plants produced fewer leaflets
If reduced gibberellin enables leaflet formation, plants forced to retain higher levels should develop fewer leaflets. This was exactly what the researchers observed.
Plants engineered to keep gibberellin active grew fewer leaflets than normal ones. Knocking out a gibberellin-breaking gene called SlGA2ox4 did the same, reducing the leaflet count.
Growth worked the other way. Plants that could not make enough gibberellin failed to expand their blades the way auxin normally would.
A further experiment linked the results. Restoring gibberellin to the blocked plants brought back the additional growth, demonstrating that gibberellin is the step through which auxin drives expansion.
Lower gibberellin levels create more leaflets
The researchers also examined the reverse situation. They reduced gibberellin activity solely in the strips between leaflets, areas in which new leaflets almost never develop.
Extra leaflets formed in those strips. Lowering gibberellin in one small zone was enough to start a leaflet where the plant would not normally produce one.
Those strips normally stay bare. Gibberellin stays high there, and that high level holds leaflets back.
The pattern appeared straightforward. A leaflet could begin wherever auxin lowered gibberellin; where gibberellin remained high, the space between leaflets stayed smooth.
A broader role in plants
This mechanism may extend beyond tomato leaves. In other plants, the same gibberellin-breaking genes become active when flowers and roots begin, locations where auxin also establishes the initial mark.
That hints at a shared step in how plants position new organs. Lower gibberellin to open a spot, then raise it to grow what fills it.
Reduced gibberellin has also been tied to the start of ovules and lateral roots in earlier work. That fits a plant-wide pattern of lowering the hormone before a new organ forms.
The switch also challenges the conventional understanding. Auxin has traditionally been regarded as a straightforward enhancer of gibberellin, but this research shows that it can initially have the opposite effect.
Questions that remain open
Several issues are still unresolved. The authors note that it is difficult to distinguish the local effects of gibberellin from its wider influence on the rate at which a whole leaf matures.
Gibberellin may also move from growing leaflets into the strips between them, keeping those strips smooth. The work points to that movement but does not show how it happens.
The Israel Science Foundation supported the work, and the authors report no competing interests.
In future, adjusting this hormonal balance might enable breeders to influence leaf shape and branching in crops. For now, that prospect requires further research.
The mechanism behind tomato leaf growth
“Our work shows that auxin achieves this by changing its conversation with gibberellin over time – first lowering gibberellin activity to allow a new organ to form and then increasing it to drive growth,” said Ori.
“This is done by affecting different target genes. This elegant two-step mechanism helps explain how plants build complex organs with remarkable precision.”
The results show how carefully timed hormone activity enables tomato plants to produce complex leaves, and could inform future crop research.
Comments
No comments yet. Be the first to comment!
Leave a Comment